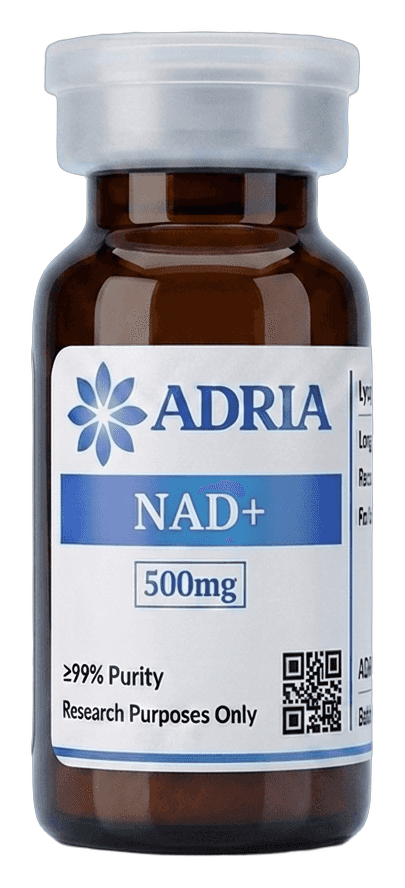
Peptide appearance
Lyophilized form helps protect peptide quality. Peptides are supplied as a dry powder, which may look like a compact "puck" or a lighter powder inside the vial.
Because the peptide is dry, it does not require refrigerated shipping during normal transit, including warm seasonal conditions. For longer storage, follow the storage guidance in the product description.
Appearance can vary. The stated peptide content is checked through third-party analysis.
Read more in the product description.
Solution not bundled
Peptides are delivered as lyophilized powder. This dry form helps preserve peptide quality during storage and transport and does not require refrigerated shipping during normal transit.
To prepare a solution, use a solvent such as Bacteriostatic water. It is sold separately, so add it only when you need it for peptide preparation.
Read more in the product description.
Longevity and Anti-aging
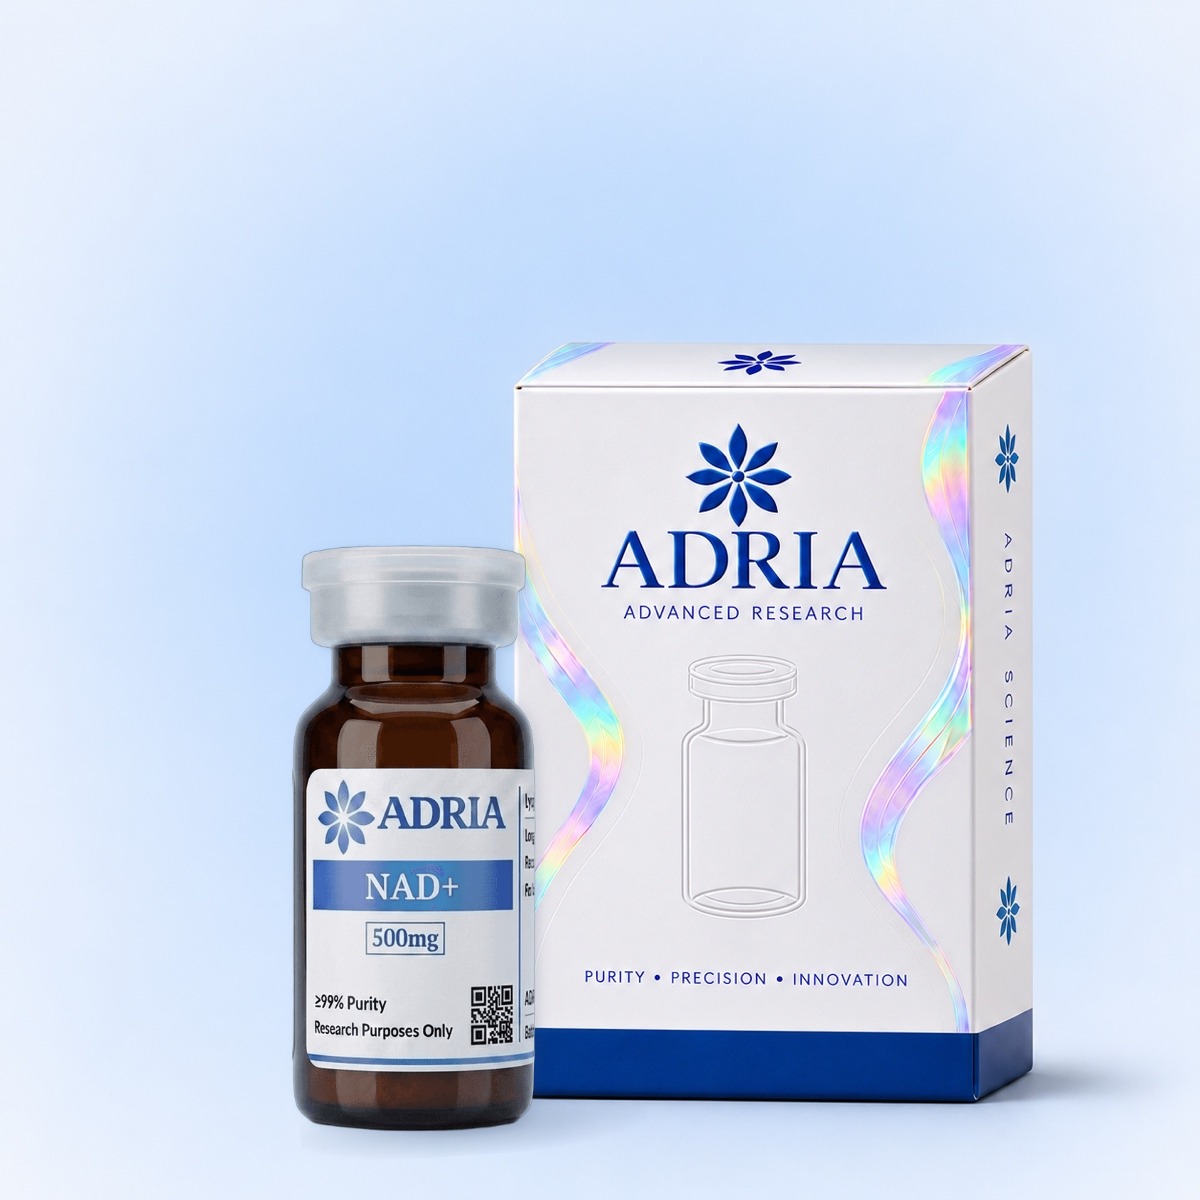
NAD+
In stock
Order within — to ship today
Arrives 26 – 30 November to Europe


 Shown at checkout
NAD+
Price range: 41,50 € through 62,50 €
NAD+ cofactor reference for redox, sirtuin, PARP, and energy-metabolism studies.
Compound information
Specifications
Molecular profile
- Molecular mass
- 663.43 g/mol
- CAS number
- 53-84-9
- Molecular formula
- C21H27N7O14P2
Material record
- Physical appearance
- White to off-white powder
- Solubility
- Soluble in bacteriostatic water and suitable aqueous laboratory solvents.
- Product note
- Nicotinamide adenine dinucleotide oxidized form; supplied strictly for research use only.
Research overview
NAD+
NAD+ levels are dynamically regulated and naturally decline with aging and under pathological conditions, thereby contributing to impaired cellular function and the acceleration of aging processes. This coenzyme was first identified in 1906 by Arthur Harden and William John Young during their investigations of alcoholic fermentation in yeast. In 1929, Harden, together with Hans von Euler-Chelpin, was awarded the Nobel Prize in Chemistry for elucidating the mechanistic role of NAD+ in mediating metabolic reactions.
At the molecular level, NAD+ functions as a central redox cofactor, undergoing cyclic interconversion between its oxidized (NAD+) and reduced (NADH) forms. This dynamic equilibrium enables electron transfer in pivotal metabolic pathways, including glycolysis, the tricarboxylic acid (Krebs) cycle, and oxidative phosphorylation. Beyond its fundamental role in mitochondrial bioenergetics, NAD+ is involved in the regulation of more than 500 enzymatic reactions, most notably through the activation of sirtuins and poly(ADP-ribose) polymerases (PARPs). Sirtuins utilize NAD+ as a substrate to modulate gene expression, epigenetic remodeling, and DNA repair, whereas PARPs depend on NAD+ to orchestrate the cellular response to DNA damage, thereby preserving genomic stability and preventing apoptosis.
Over the past decades, research has underscored the pleiotropic effects of NAD+ extending far beyond energy metabolism. Elevated NAD+ levels correlate with enhanced muscle strength, increased endurance, and neuroprotection. Moreover, NAD+ contributes to the activation of the transcriptional coactivator PGC-1α, which safeguards neurons against oxidative stress and has been associated with improved cognitive performance in aging.
Research Confirmed Effects
One of the hallmarks of physiological aging is the progressive decline in mitochondrial function, manifested by reduced ATP production, disrupted redox homeostasis, and accumulation of reactive oxygen species. This phenomenon is closely associated with cellular senescence, chronic inflammation, and diminished regenerative capacity of stem cells. NAD+ levels naturally decrease with age, leading to impaired nuclear–mitochondrial communication and the development of a so-called pseudohypoxic state, which accelerates tissue and organ dysfunction. The consequence is reduced cellular resilience to stress and increased susceptibility to degenerative processes.
Experimental studies have demonstrated that supplementation with NAD+ precursors (e.g., nicotinamide riboside or nicotinamide mononucleotide) can restore mitochondrial bioenergetics and improve signaling between the nucleus and mitochondria. A key mechanism involves the activation of NAD+-dependent enzymes, particularly sirtuins (SIRT1) and poly(ADP-ribose) polymerases (PARPs). Activation of SIRT1 enhances the expression of longevity-associated genes, regulates metabolic pathways, and mitigates inflammatory responses. Restoration of mitochondrial integrity through NAD+ has been linked to improvements in muscle strength, endurance, and neuroprotection, underscoring its therapeutic potential in preventing age-related pathologies.
Beyond its bioenergetic and genomic effects, NAD+ exerts pleiotropic influences on organismal homeostasis. It contributes to the regulation of circadian rhythms, immune responses, and the maintenance of vascular elasticity. Experimental models have shown that elevating NAD+ levels can protect against atherosclerotic changes, support neural tissue regeneration, and enhance cognitive performance in advanced age. Collectively, these findings suggest that targeted augmentation of NAD+ represents a promising anti-aging strategy capable of slowing or partially reversing aging processes and extending the period of functional vitality.
The decline in NAD+ levels represents a critical factor influencing the aging of skeletal muscle. With advancing age, mitochondrial bioenergetics progressively deteriorates, oxidative phosphorylation is reduced, and the accumulation of reactive oxygen species increases. This cascade results in the loss of muscle mass, diminished contractile capacity, and impaired regenerative potential of muscle tissue. A key mechanism involves the disruption of nuclear–mitochondrial communication, leading to a pseudohypoxic state characteristic of advanced muscle dysfunction. Early intervention through NAD+ supplementation or its precursors can restore mitochondrial homeostasis and delay the onset of irreversible alterations.
Experimental studies indicate that supplementation with NAD+ precursors, such as nicotinamide mononucleotide (NMN) and nicotinamide riboside (NR), improves mitochondrial function and enhances the expression of genes linked to oxidative metabolism. Central to this effect is the activation of NAD+-dependent enzymes, most notably sirtuin 1 (SIRT1), which regulates gene transcription and maintains mitochondrial DNA integrity. Activation of these pathways supports the preservation of muscle contractile performance, augments resistance to oxidative stress, and mitigates degenerative processes associated with aging.
Beyond pharmacological interventions, regular physical activity has been shown to exert comparable effects on mitochondrial homeostasis to NAD+ supplementation. Exercise increases levels of PGC-1α, a transcriptional coactivator that drives mitochondrial biogenesis and angiogenesis within muscle tissue. The combination of endurance training and NAD+ precursor supplementation thus represents a promising strategy to synergistically attenuate age-related muscle loss, enhance metabolic flexibility, and sustain long-term skeletal muscle vitality throughout the aging process.
Alterations in NAD+ levels have emerged as a critical factor in the onset and progression of neurodegenerative disorders. A decline in this coenzyme disrupts mitochondrial bioenergetics, exacerbates oxidative stress, and reduces neuronal resilience against injury. Such perturbations are closely associated with progressive neurodegeneration observed in Alzheimer’s disease, Parkinson’s disease, and Huntington’s disease. Mitochondrial dysfunction, in conjunction with excessive production of reactive oxygen species (ROS), accelerates neuronal damage and promotes chronic neuroinflammation, which constitutes a hallmark of age-related neurological decline.
Experimental evidence indicates that supplementation with NAD+ precursors, such as nicotinamide riboside (NR) and nicotinamide mononucleotide (NMN), exerts robust neuroprotective effects. These interventions enhance oxidative phosphorylation, stabilize mitochondrial DNA, and activate NAD+-dependent enzymes, including sirtuins and poly(ADP-ribose) polymerases (PARPs). In particular, SIRT1 and SIRT3 orchestrate transcriptional programs that preserve mitochondrial integrity, attenuate inflammatory signaling, and enhance neuronal survival. Restoration of NAD+ levels has been shown to mitigate motor deficits and prevent dopaminergic neuronal loss in Parkinsonian models, while also ameliorating bioenergetic deficits associated with Huntington’s disease.
An additional dimension involves the kynurenine pathway of tryptophan metabolism. Under pathological conditions, dysregulation of this pathway diverts tryptophan away from neurotransmitter biosynthesis toward NAD+ production, thereby reducing the availability of serotonin and other essential metabolites. Imbalances in kynurenine-derived metabolites have been consistently linked not only to neurodegenerative diseases but also to psychiatric disorders. This underscores the notion that maintaining homeostasis in NAD+ and tryptophan metabolism may be essential for preventing or slowing neurodegenerative progression. Consequently, NAD+ supplementation or targeted modulation of the kynurenine pathway represents a promising therapeutic approach for preserving neuronal function.
A decline in NAD+ levels is closely linked to the dysregulation of nicotinamide phosphoribosyltransferase (NAMPT), a key enzyme in NAD+ biosynthesis that also functions as a potent mediator of inflammation. Under conditions of NAD+ depletion, NAMPT becomes aberrantly activated, thereby driving pro-inflammatory signaling pathways and increasing the risk of metabolic disorders such as obesity, type 2 diabetes mellitus, and non-alcoholic fatty liver disease. Moreover, NAMPT is frequently overexpressed in tumor cells, where it promotes cellular proliferation and survival, rendering it a promising target for antineoplastic therapies.
Available evidence suggests that supplementation with NAD+ or its precursors may attenuate pathological NAMPT activation, thereby contributing to the modulation of inflammatory responses. The balance between NAD+ and NAMPT represents a critical determinant of insulin sensitivity; disruption of this axis leads to enhanced lipolysis, accumulation of circulating free fatty acids, and impaired glucose metabolism in both liver and skeletal muscle. Restoring NAD+ homeostasis therefore emerges as a viable strategy to improve metabolic regulation, reduce inflammatory burden, and prevent chronic age-associated diseases.
Substance use disorders, including chronic alcohol consumption and drug dependence, have long been associated with a decline in NAD+ levels, leading to impaired cellular bioenergetics and secondary nutritional deficiencies. These biochemical perturbations are tightly linked to dysregulation of neurotransmitter systems, manifesting as mood disturbances, cognitive dysfunction, and heightened vulnerability to stress.
As early as the 1960s, initial therapeutic attempts employing intravenous NAD+ administration in alcohol-dependent patients demonstrated improvements in withdrawal symptoms as well as restoration of metabolic homeostasis. According to subsequent scientific observations, NAD+ should be regarded as a pivotal cofactor that not only replenishes energy balance but also modulates neurochemical pathways implicated in the initiation, maintenance, and progression of addictive behaviors.
Conclusion
Experimental models have demonstrated that NAD+ exerts vasoprotective effects by mitigating atherosclerotic changes and preserving aortic elasticity. Furthermore, as an extracellular signaling molecule, NAD+ facilitates communication between neurons and smooth muscle cells, thereby influencing gastrointestinal motility and contributing to the regulation of vascular tone and blood pressure. Given the age-associated decline in NAD+ availability, current research on its precursors, including nicotinamide riboside (NR) and nicotinamide mononucleotide (NMN), highlights promising therapeutic avenues aimed at decelerating aging processes and sustaining cellular vitality.
For laboratory purposes and personal observation only. Not for human consumption.
Laboratory care
Handling
Product storage
Sealed dry material: store at -20 °C, dry and protected from light. Prepared solutions require a laboratory-validated stability protocol.
Material in transport
Keep the sealed container dry, protected from direct light, and within the product-specific laboratory transport conditions.
Storage of dry material
Keep the sealed reference material protected from moisture and light and follow the product-specific storage record maintained by Adria Science.
Storage of prepared laboratory solutions
Prepared laboratory solutions require compatible solvent selection, clean handling, and a documented laboratory stability policy.
Analytical documentation
Tests
Documentation is available on request
Contact us for the current record for this strength. We never substitute a generic or mismatched certificate.
Your batch is confirmed when your order is allocated.Latest published result
Liquilabs s.r.o.Signed Certificate of Analysis · 500mg
98.9%Purity by HPLC
Recorded QC panel
- AssayPeptide screening
- 418 mg
- PurityPeptide screening
- 98.9%
- Identity (FTIR)FTIR spectrum
- 1000
- Identity (RT)Retention time
- 0.987
These are the latest published results for this strength. The batch number is printed on each vial. Your supplied batch is confirmed against the matching published record when your order is allocated.
Source record
References
“NAD+ Science 101 - What Is NAD+ & Why It’s Important,” Elysium Health. [Online]. Available: https://www.elysiumhealth.com/en-us/knowledge/science-101/everything-you-need-to-know-about-nicotinamide-adenine-dinucleotide-nad. [Accessed: 25-Jul-2019].
“Nicotinamide Riboside: Benefits, Side Effects and Dosage,” Healthline. [Online]. Available: https://www.healthline.com/nutrition/nicotinamide-riboside. [Accessed: 25-Jul-2019].
R. T. Matthews, L. Yang, S. Browne, M. Baik, and M. F. Beal, “Coenzyme Q10 administration increases brain mitochondrial concentrations and exerts neuroprotective effects,” Proc. Natl. Acad. Sci. U. S. A., vol. 95, no. 15, pp. 8892–8897, Jul. 1998. [PMC]
“What You Need to Know About Resveratrol Supplements,” WebMD. [Online]. Available: https://www.webmd.com/heart-disease/resveratrol-supplements. [Accessed: 25-Jul-2019].
N. Sun, R. J. Youle, and T. Finkel, “The Mitochondrial Basis of Aging,” Mol. Cell, vol. 61, no. 5, pp. 654–666, Mar. 2016. [PMC]
D. Stipp, “Beyond Resveratrol: The Anti-Aging NAD Fad,” Scientific American Blog Network. [Online]. Available: https://blogs.scientificamerican.com/guest-blog/beyond-resveratrol-the-anti-aging-nad-fad/. [Accessed: 08-Jul-2019].
A. P. Gomes et al., “Declining NAD+ Induces a Pseudohypoxic State Disrupting Nuclear-Mitochondrial Communication during Aging,” Cell, vol. 155, no. 7, pp. 1624–1638, Dec. 2013. [PMC]
S. Imai and L. Guarente, “NAD+ and sirtuins in aging and disease,” Trends Cell Biol., vol. 24, no. 8, pp. 464–471, Aug. 2014. [PubMed]
A. R. Mendelsohn and J. W. Larrick, “Partial reversal of skeletal muscle aging by restoration of normal NAD+ levels,” Rejuvenation Res., vol. 17, no. 1, pp. 62–69, Feb. 2014. [PubMed]
C. Kang, E. Chung, G. Diffee, and L. L. Ji, “Exercise training attenuates aging-associated mitochondrial dysfunction in rat skeletal muscle: role of PGC-1α,” Exp. Gerontol., vol. 48, no. 11, pp. 1343–1350, Nov. 2013. [PubMed]
S. Ringholm et al., “Effect of lifelong resveratrol supplementation and exercise training on skeletal muscle oxidative capacity in aging mice; impact of PGC-1α,” Exp. Gerontol., vol. 48, no. 11, pp. 1311–1318, Nov. 2013. [PubMed]
A. Lloret and M. F. Beal, “PGC-1α, Sirtuins and PARPs in Huntington’s Disease and Other Neurodegenerative Conditions: NAD+ to Rule Them All,” Neurochem. Res., May 2019. [PubMed]
C. Shan et al., “Protective effects of β- nicotinamide adenine dinucleotide against motor deficits and dopaminergic neuronal damage in a mouse model of Parkinson’s disease,” Prog. Neuropsychopharmacol. Biol. Psychiatry, vol. 94, p. 109670, Jun. 2019. [PubMed]
D. C. Maddison and F. Giorgini, “The kynurenine pathway and neurodegenerative disease,” Semin. Cell Dev. Biol., vol. 40, pp. 134–141, Apr. 2015. [PubMed]
A. Garten, S. Schuster, M. Penke, T. Gorski, T. de Giorgis, and W. Kiess, “Physiological and pathophysiological roles of NAMPT and NAD metabolism,” Nat. Rev. Endocrinol., vol. 11, no. 9, pp. 535–546, Sep. 2015. [PubMed]
S. Yamaguchi and J. Yoshino, “Adipose Tissue NAD+ Biology in Obesity and Insulin Resistance: From Mechanism to Therapy,” BioEssays News Rev. Mol. Cell. Dev. Biol., vol. 39, no. 5, May 2017. [PMC]
J. E. Humiston, “Nicotinamide Adenine Dinucleotide,” p. 68. [FDA]
National Center for Biotechnology Information
PubChem Compound Summary: Nicotinamide adenine dinucleotide
Authoritative identity record for oxidized NAD+.
PubChem View source ↗Chemical Abstracts Service
CAS Common Chemistry: 53-84-9
Authoritative CAS Registry Number record for NAD+.
CAS Common Chemistry View source ↗Cantó C, Gerhart-Hines Z, Feige JN, et al. · 2009
AMPK regulates energy expenditure by modulating NAD+ metabolism and SIRT1 activity
Primary report on NAD+-linked metabolic signalling.
Nature · 10.1038/nature07813 View source ↗Koneshamoorthy A, Seniveratne-Epa D, Calder G, Sawyer M, Kay TWH, Farrell S, Loudovaris T, Mariana L, McCarthy D, Lyu R, Liu X, Thorn P, Tong J, Chin LK, Zacharin M, Trainer A, Taylor S, MacIsaac RJ, Sachithanandan N, Thomas HE, Krishnamurthy B · 2022
Case Report: Hypoglycemia Due to a Novel Activating Glucokinase Variant in an Adult - a Molecular Approach
Frontiers in endocrinology View source ↗Imai S, Guarente L · 2014
NAD+ and sirtuins in aging and disease
Trends in cell biology View source ↗Diaz-Mejia JJ, Meng EC, Pico AR, MacParland SA, Ketela T, Pugh TJ, Bader GD, Morris JH · 2019
Evaluation of methods to assign cell type labels to cell clusters from single-cell RNA-sequencing data
F1000Research View source ↗Abdellatif M, Sedej S, Kroemer G · 2021
NAD(+) Metabolism in Cardiac Health, Aging, and Disease
Circulation View source ↗Katsyuba E, Romani M, Hofer D, Auwerx J · 2020
NAD(+) homeostasis in health and disease
Nature metabolism View source ↗Kane AE, Sinclair DA · 2018
Sirtuins and NAD(+) in the Development and Treatment of Metabolic and Cardiovascular Diseases
Circulation research View source ↗Customer reviews

Quality products,fast shipping,great refferal plan,only downside is that products in 4 mounths since my first order got more and more expensive ,but overall verry good experience.
Read full review →More than 2 weeks for package dispatch. They promised one free peptide next time. Sent me new tracking number but package still wasn't delivered to fedex. Last package (much much cheaper) was delivered in less than week. I will update if they will send my package. ok,package sent.
Read full review →Extremely satisfied with the product quality and overall experience. The customer service is polite and quick. All recommendations!
Read full review →Great service!
Read full review →Always on time and customer care is super great
Read full review →Fast good, and quality is perfect
Read full review →ordered 3 times now and everything ok every time.
Read full review →Trustworthy site with a huge catalog of products. Been purchasing from them for some time now never got disappointed. I could only recommend them.
Read full review →Great quality product
Read full review →Everything was great, super customer support, honest, reliable
Read full review →Everything ok. With little problem with package, but after contact with Customer Service everything went right. Good quality of products
Read full review →Excellent. Buying peptides online can be nerve wracking! But Adria are very transparent about all the checks and certifications. My experience with them was excellent. Great products at good prices and efficient P&P
Read full review →Continue exploring